По2
Сообщений 751 страница 762 из 762
Поделиться75114-08-2026 14:52:08
- Активный участник

- Зарегистрирован: 06-07-2011
- Сообщений: 17394
- Пол: Мужской
- Возраст: 68 [1958-05-12]
- Провел на форуме:
3 месяца 13 дней - Последний визит:
Сегодня 16:37:34
Поделиться75218-08-2026 19:57:08
- Активный участник

- Зарегистрирован: 25-07-2011
- Сообщений: 13988
- Провел на форуме:
4 месяца 19 дней - Последний визит:
02-09-2026 08:45:14

Поделиться75318-08-2026 20:00:06
- Администратор

- Откуда: Sol III
- Зарегистрирован: 30-07-2011
- Сообщений: 52239
- Пол: Мужской
- Провел на форуме:
1 год 4 месяца - Последний визит:
Сегодня 22:04:10

рот до ушей, хоть завязочки пришей )))
Поделиться75418-08-2026 23:44:02
- Активный участник
- Зарегистрирован: 25-07-2011
- Сообщений: 13988
- Провел на форуме:
4 месяца 19 дней - Последний визит:
02-09-2026 08:45:14


Поделиться75527-08-2026 22:01:21
- Активный участник
- Зарегистрирован: 25-07-2011
- Сообщений: 13988
- Провел на форуме:
4 месяца 19 дней - Последний визит:
02-09-2026 08:45:14
Отредактировано Au (27-08-2026 22:02:07)
Поделиться75627-08-2026 22:03:09
- Активный участник
- Зарегистрирован: 25-07-2011
- Сообщений: 13988
- Провел на форуме:
4 месяца 19 дней - Последний визит:
02-09-2026 08:45:14
Поделиться75727-08-2026 22:55:12
- Активный участник
- Зарегистрирован: 25-07-2011
- Сообщений: 13988
- Провел на форуме:
4 месяца 19 дней - Последний визит:
02-09-2026 08:45:14
Поделиться75828-08-2026 00:00:13
- Администратор
- Откуда: Sol III
- Зарегистрирован: 30-07-2011
- Сообщений: 52239
- Пол: Мужской
- Провел на форуме:
1 год 4 месяца - Последний визит:
Сегодня 22:04:10
была такая, ага..
а еще была нототения - вот куда она делась?.. 
Поделиться75928-08-2026 00:06:04
- Администратор
- Откуда: Sol III
- Зарегистрирован: 30-07-2011
- Сообщений: 52239
- Пол: Мужской
- Провел на форуме:
1 год 4 месяца - Последний визит:
Сегодня 22:04:10
и шо же это за водила такой, у которого было НЕСКОЛЬКО ДЕСЯТКОВ возможных ДТП, от которых его спасал только этот ыскусственный, простихоссспади, ынтилехт?.. 
Поделиться76028-08-2026 11:32:46
- Активный участник
- Зарегистрирован: 25-07-2011
- Сообщений: 13988
- Провел на форуме:
4 месяца 19 дней - Последний визит:
02-09-2026 08:45:14
Это все водилы
Была и в натотения
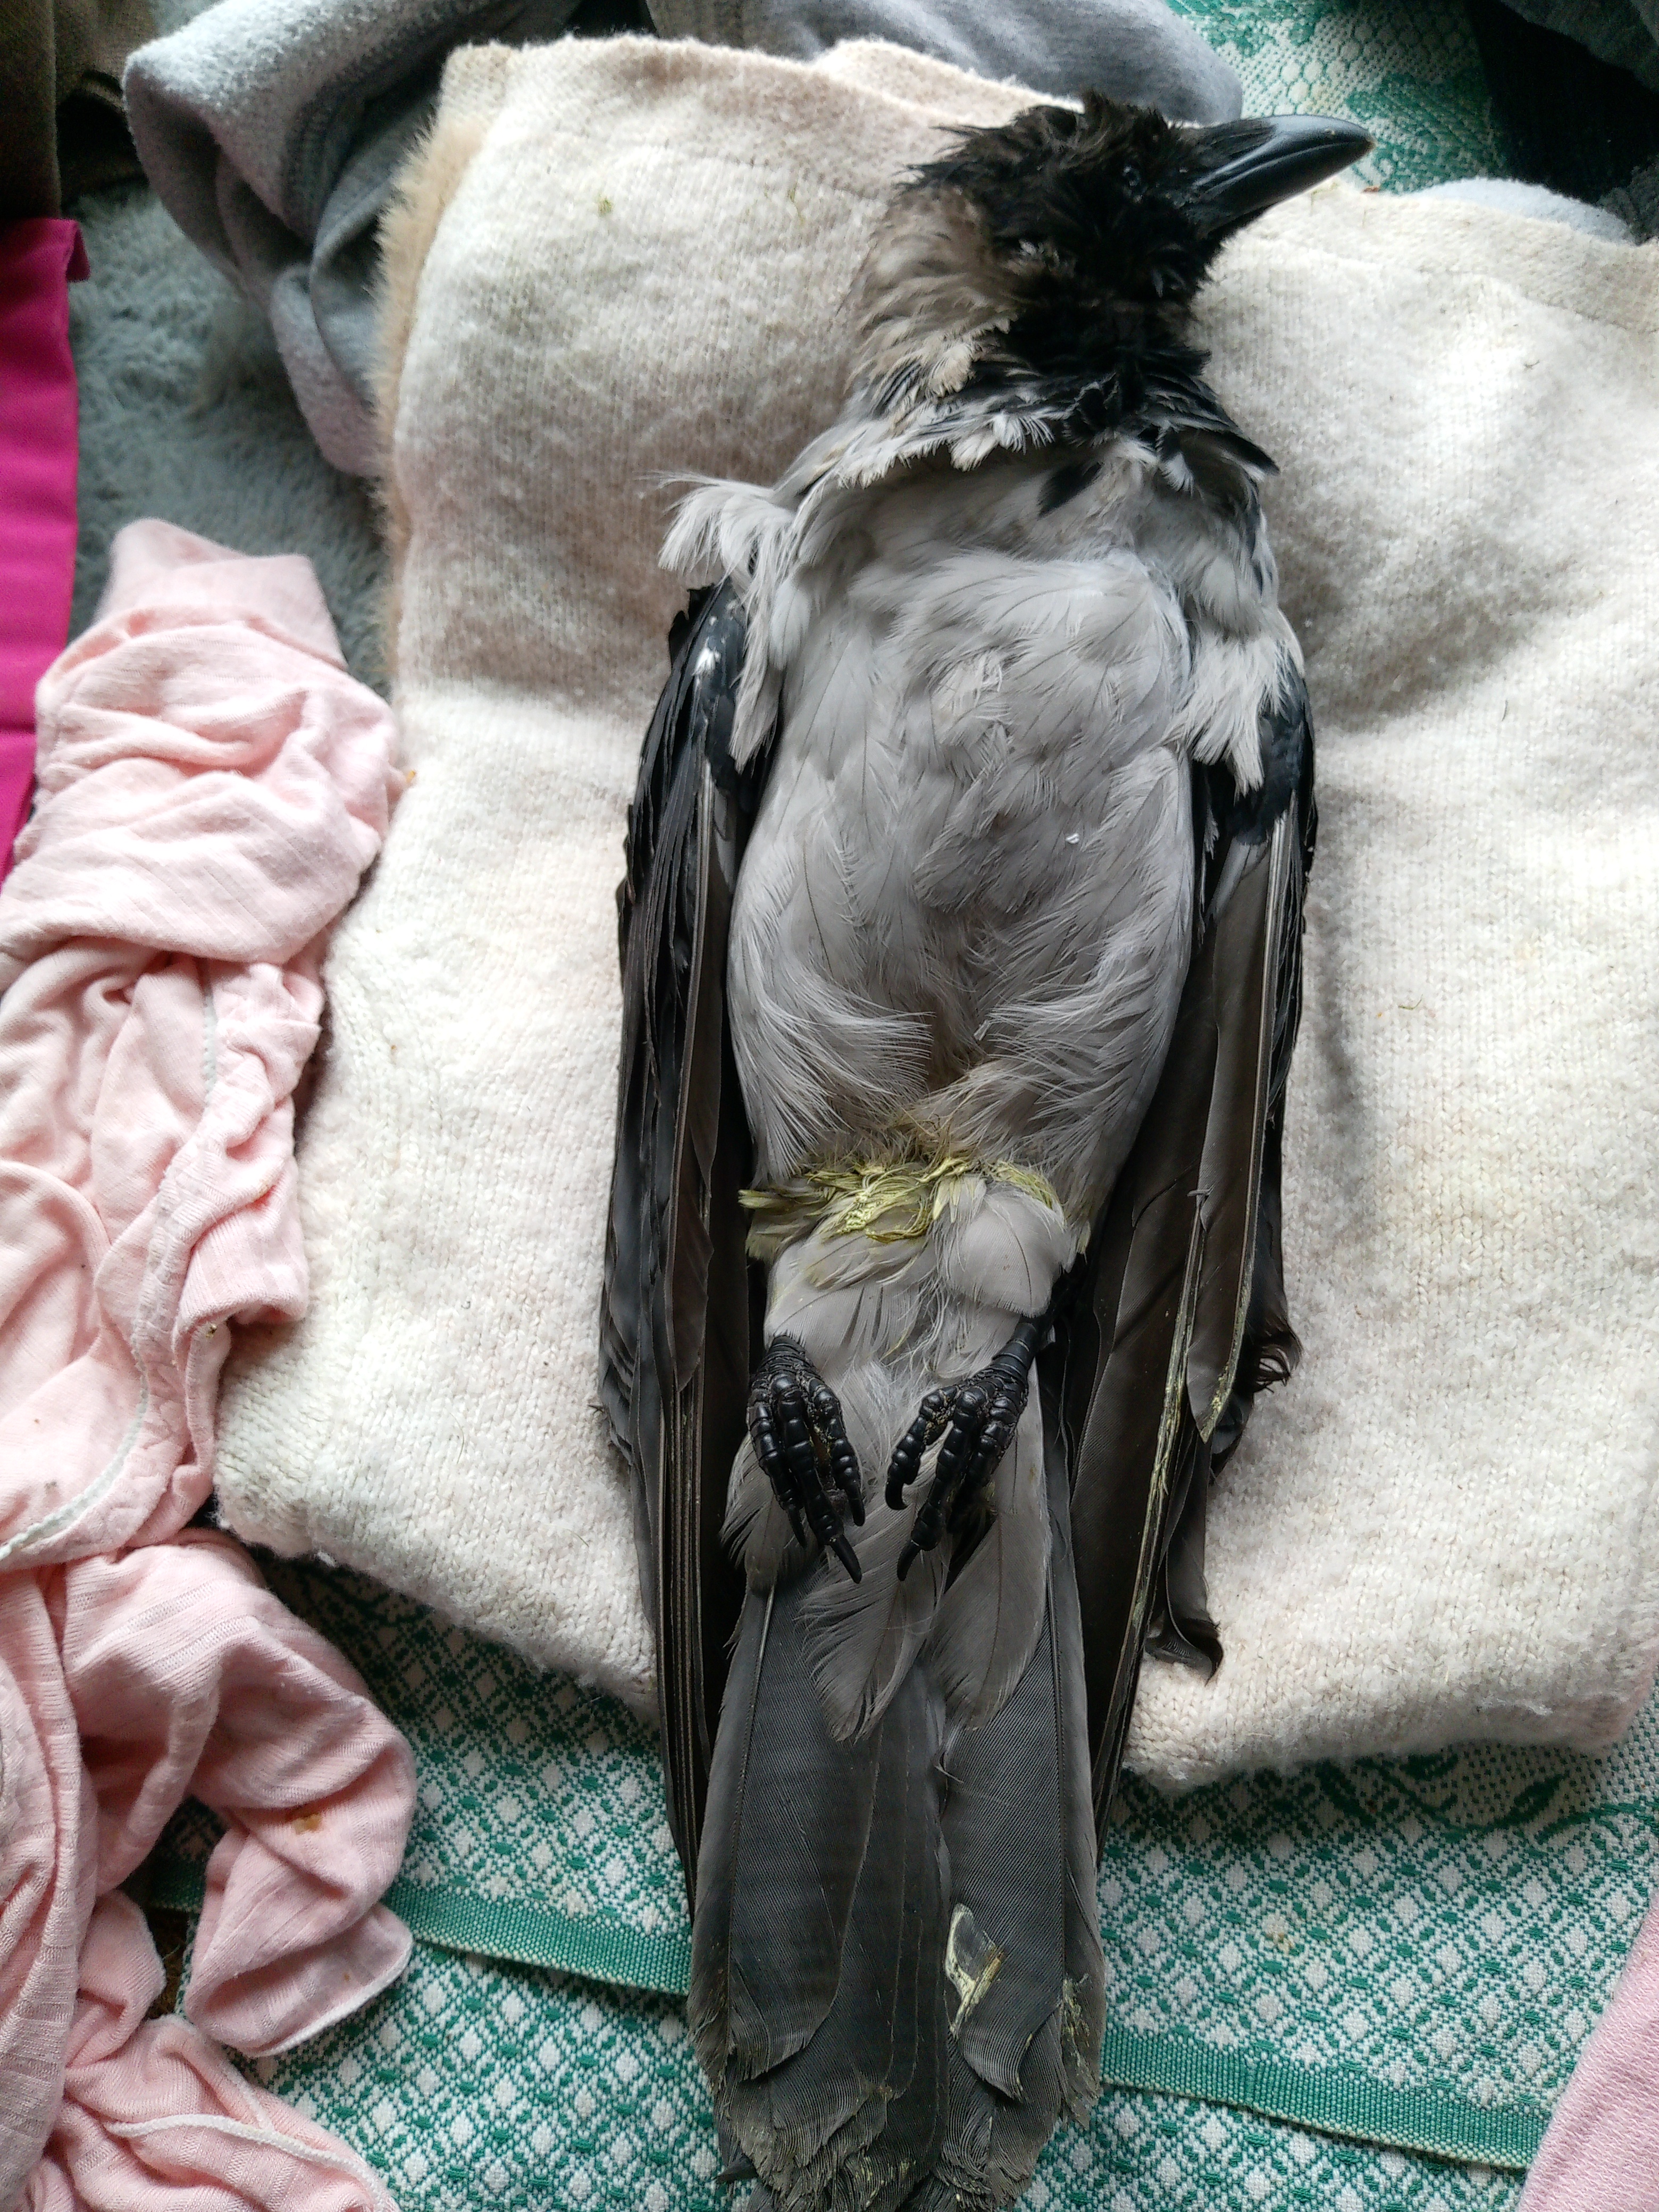
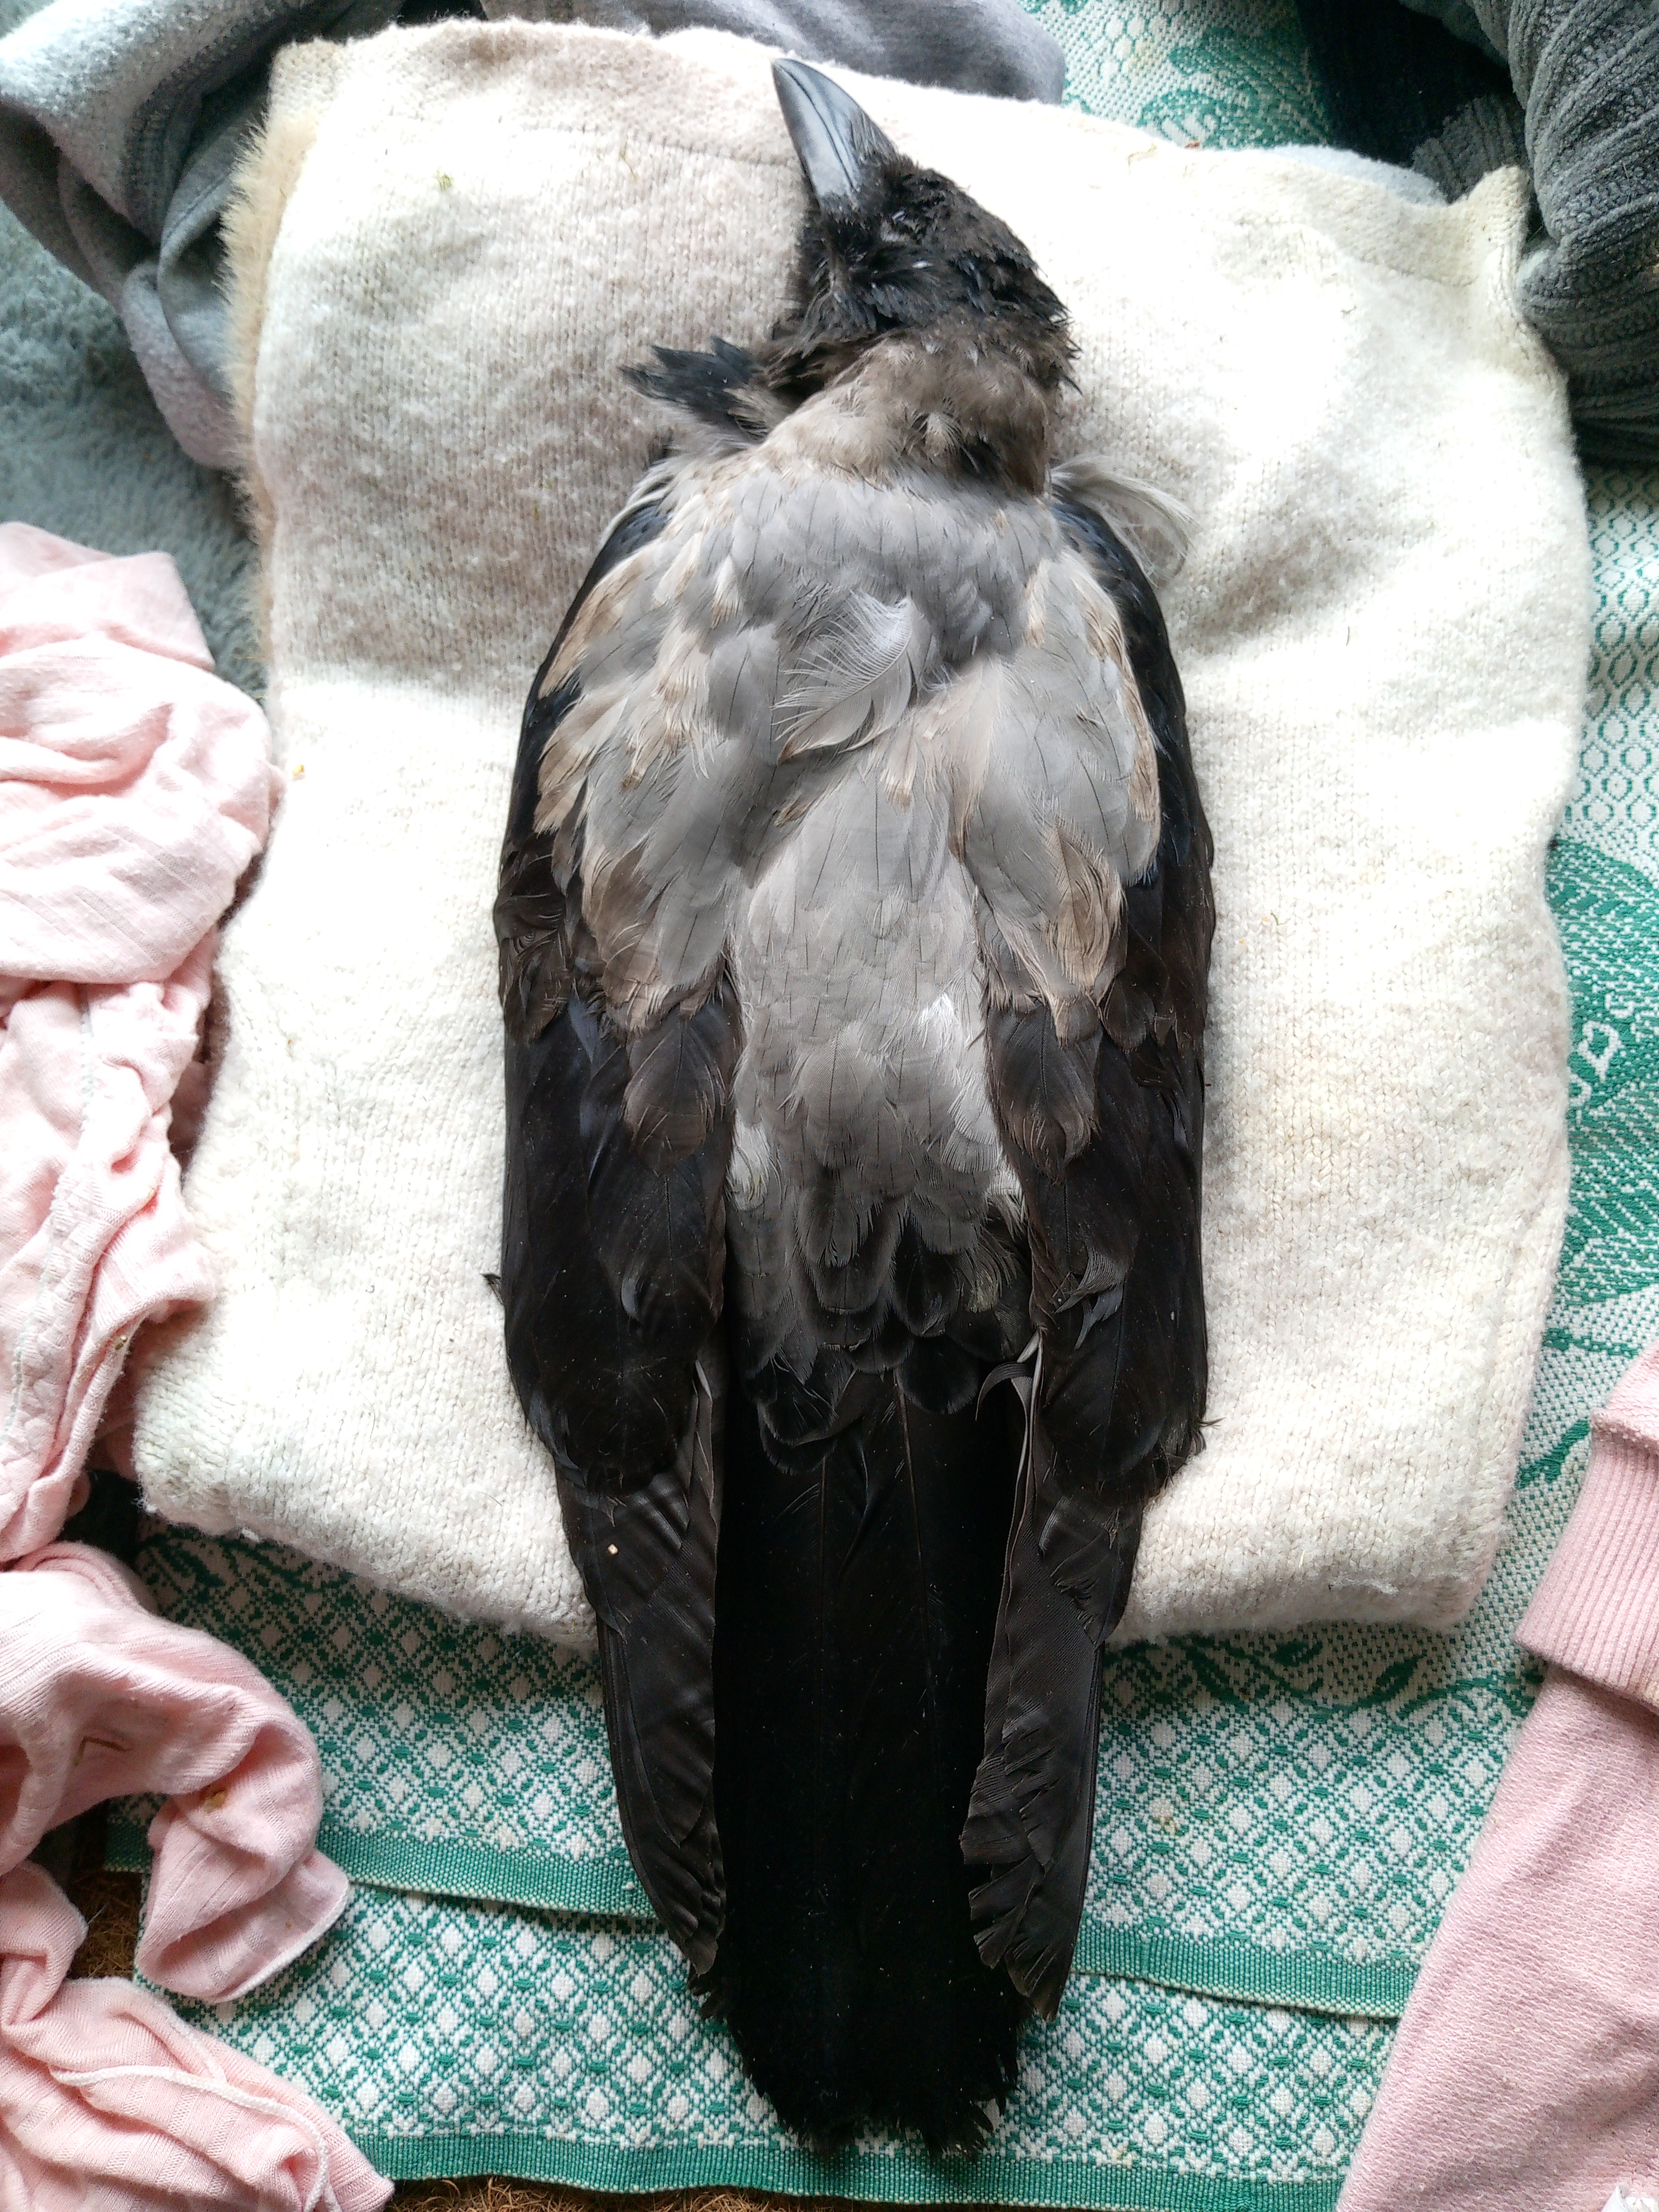
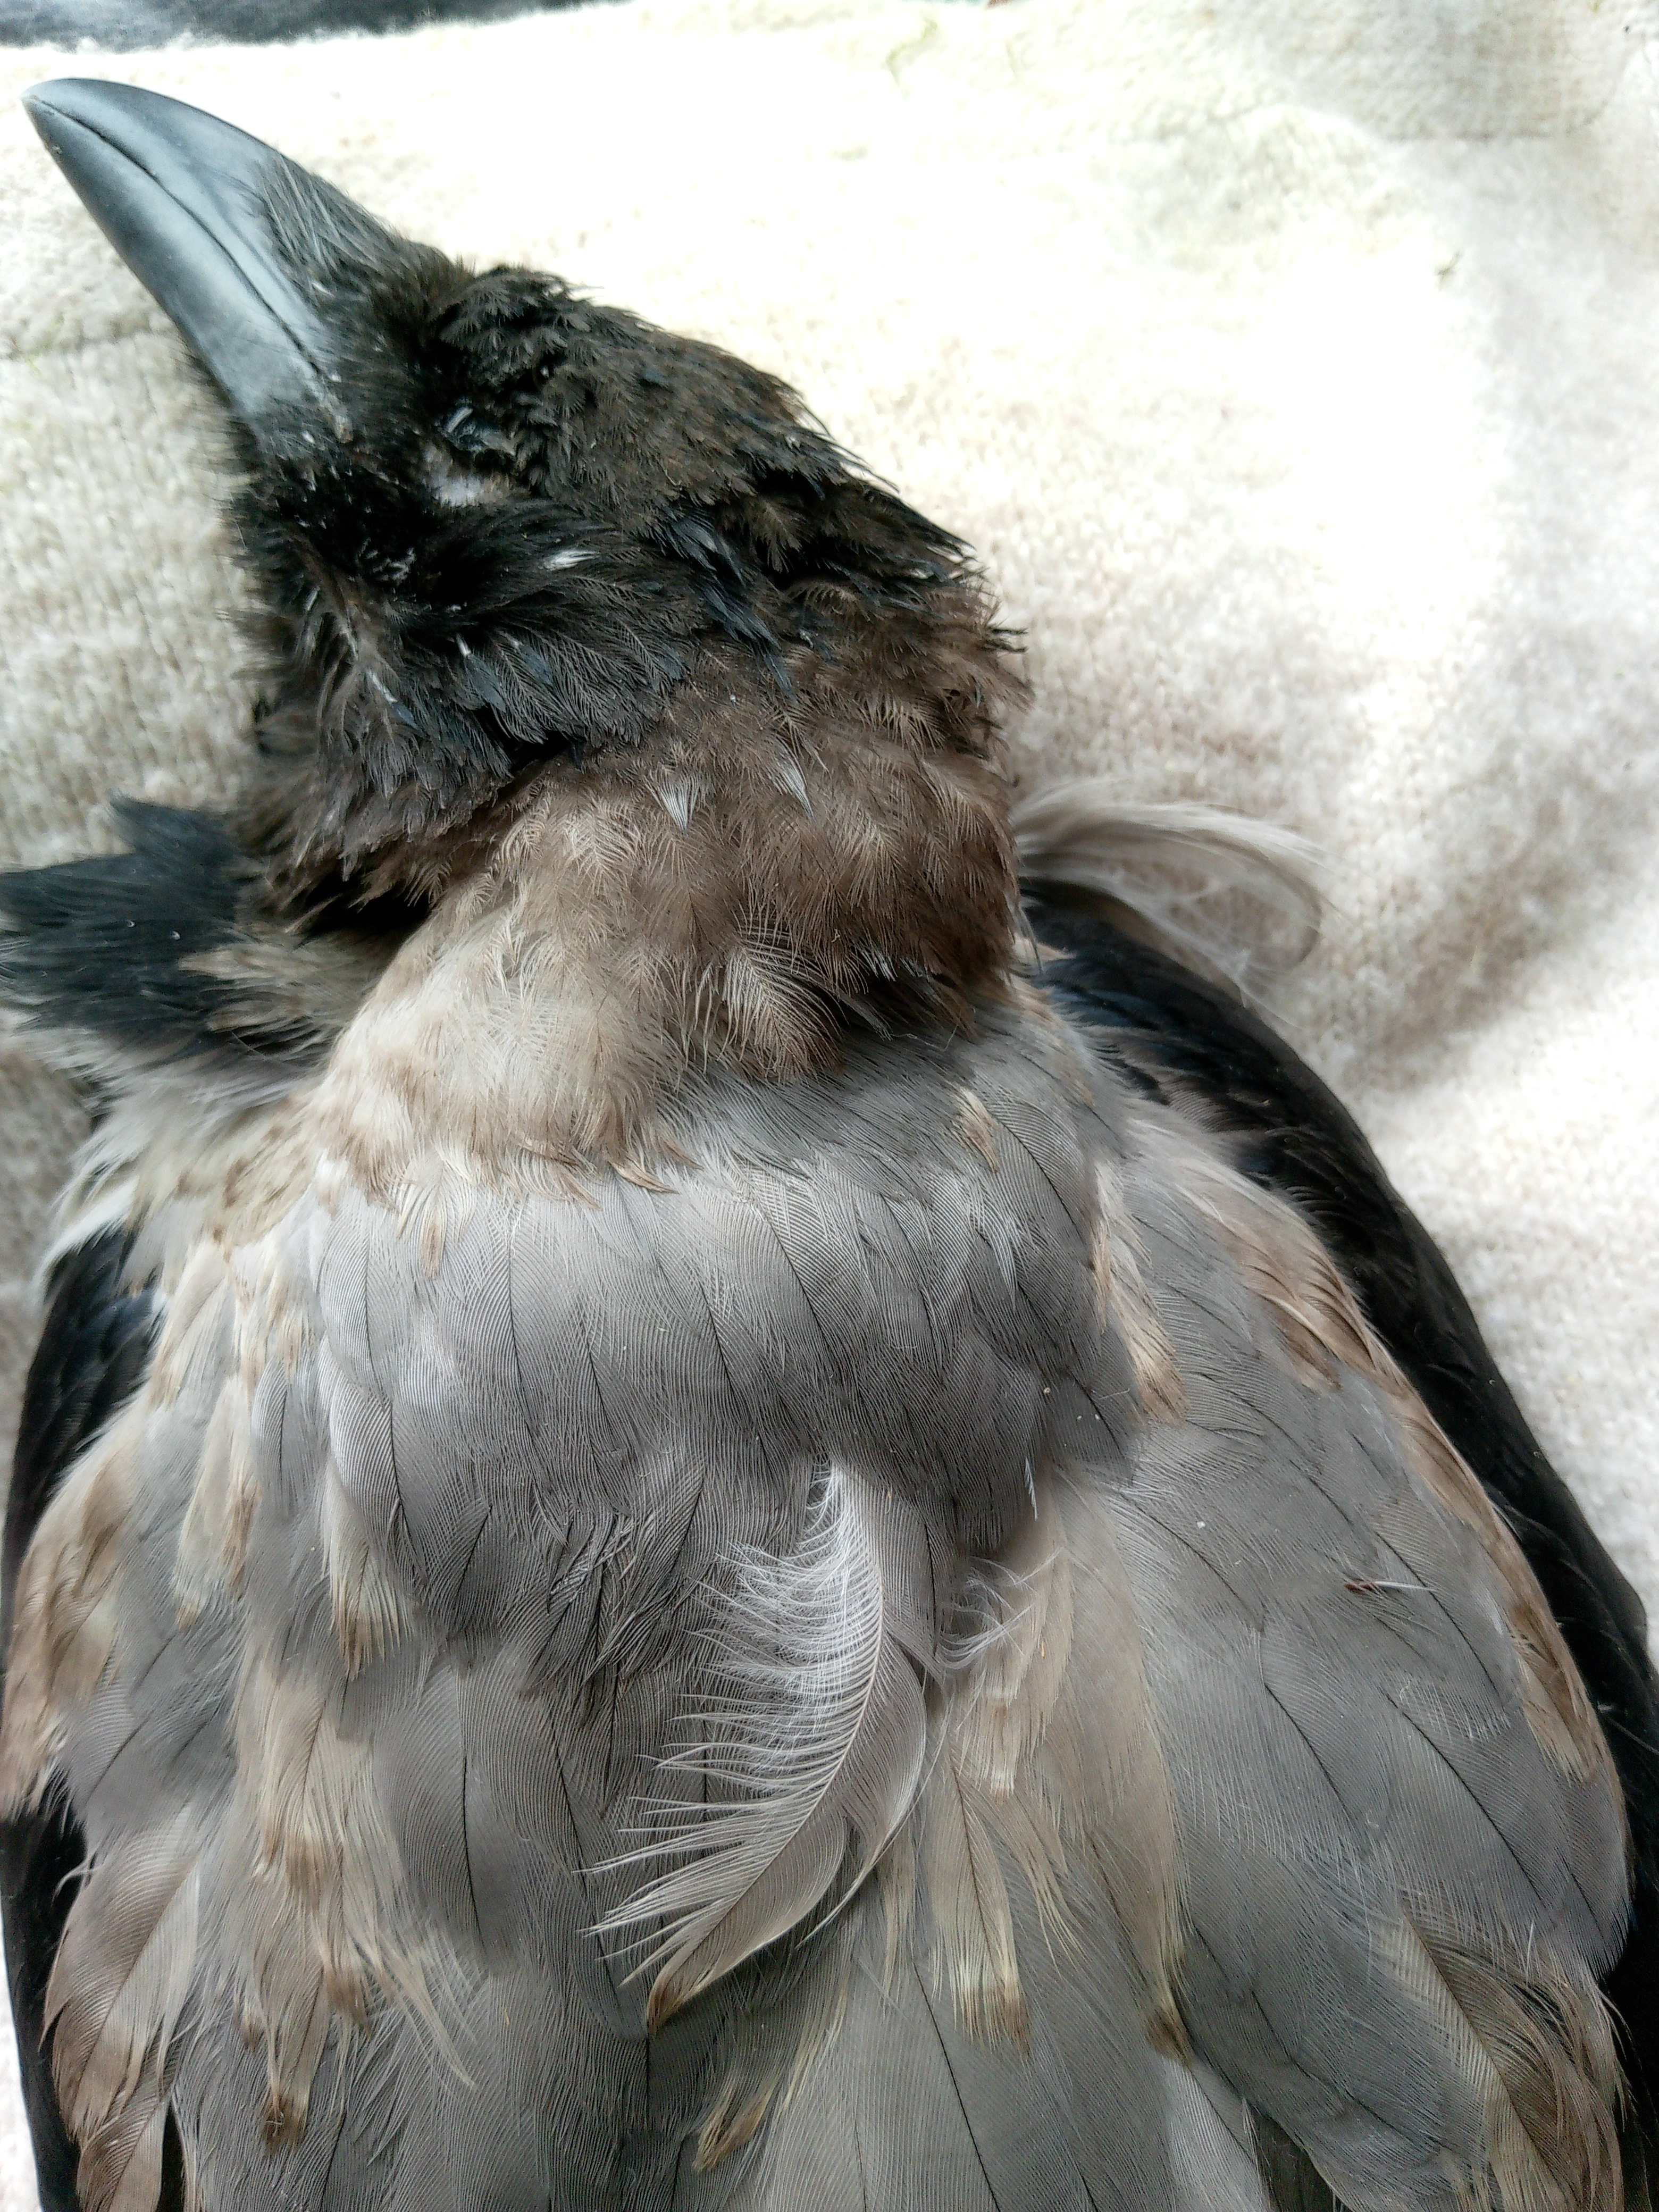
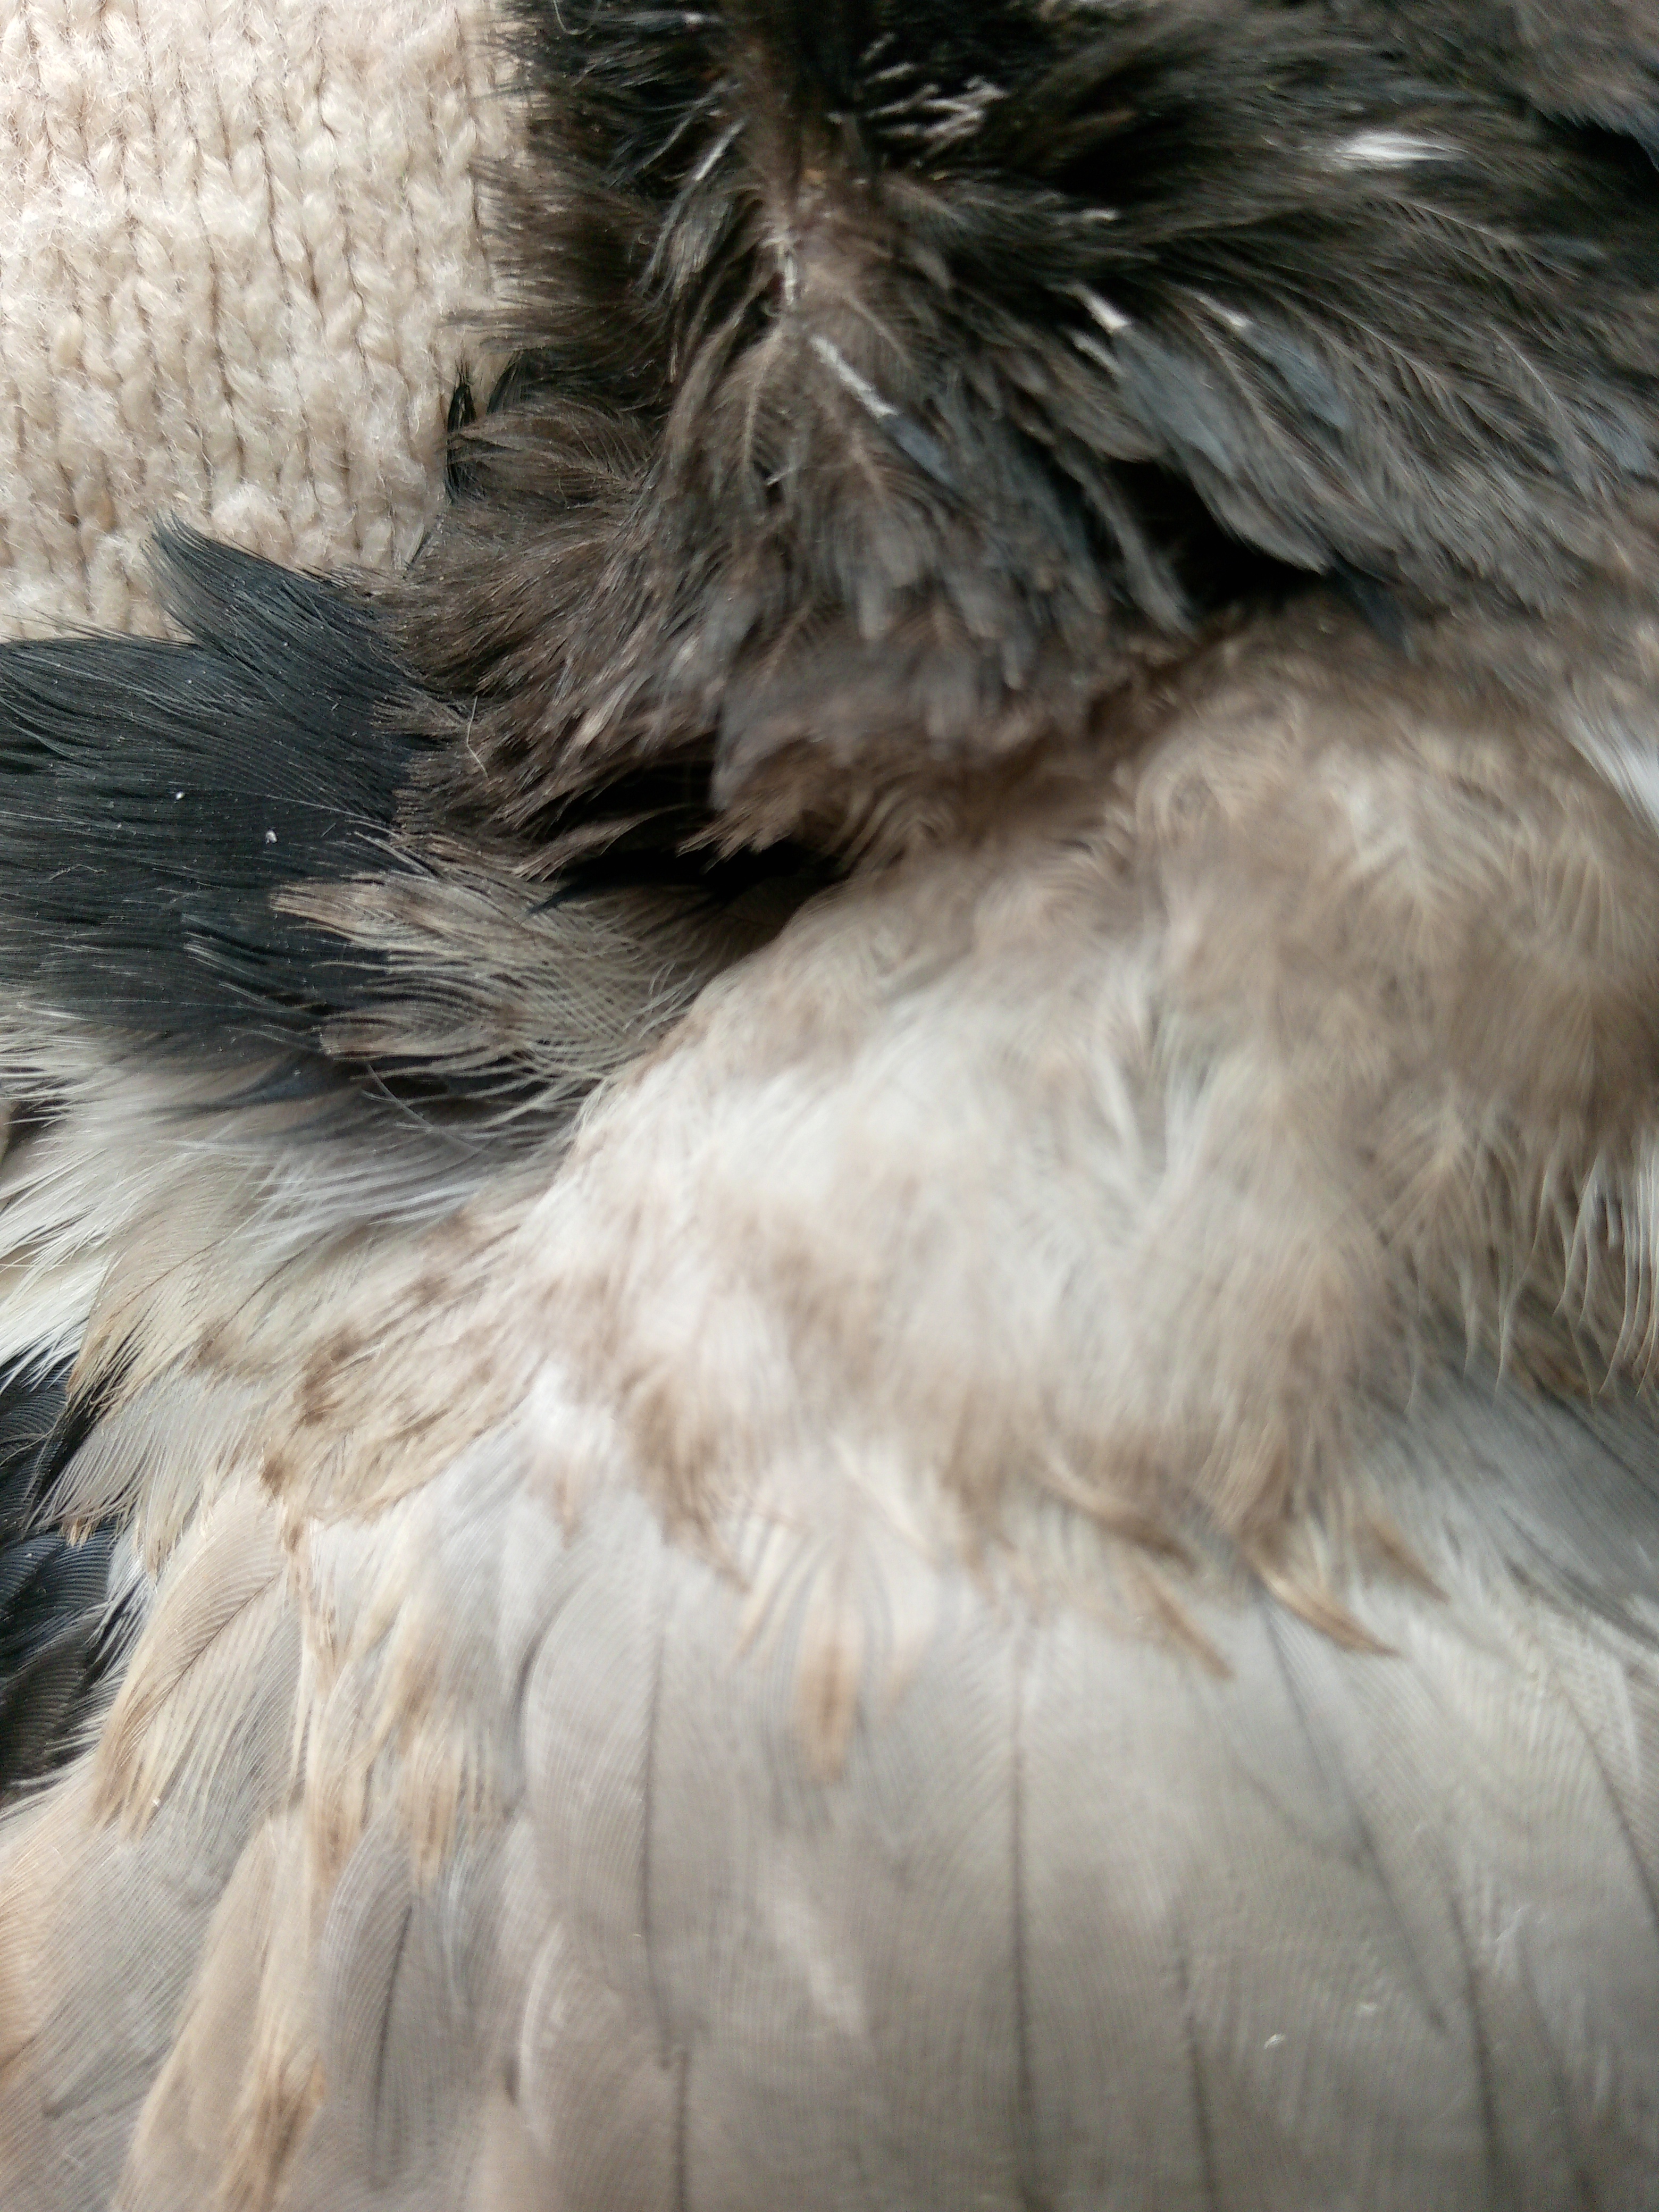
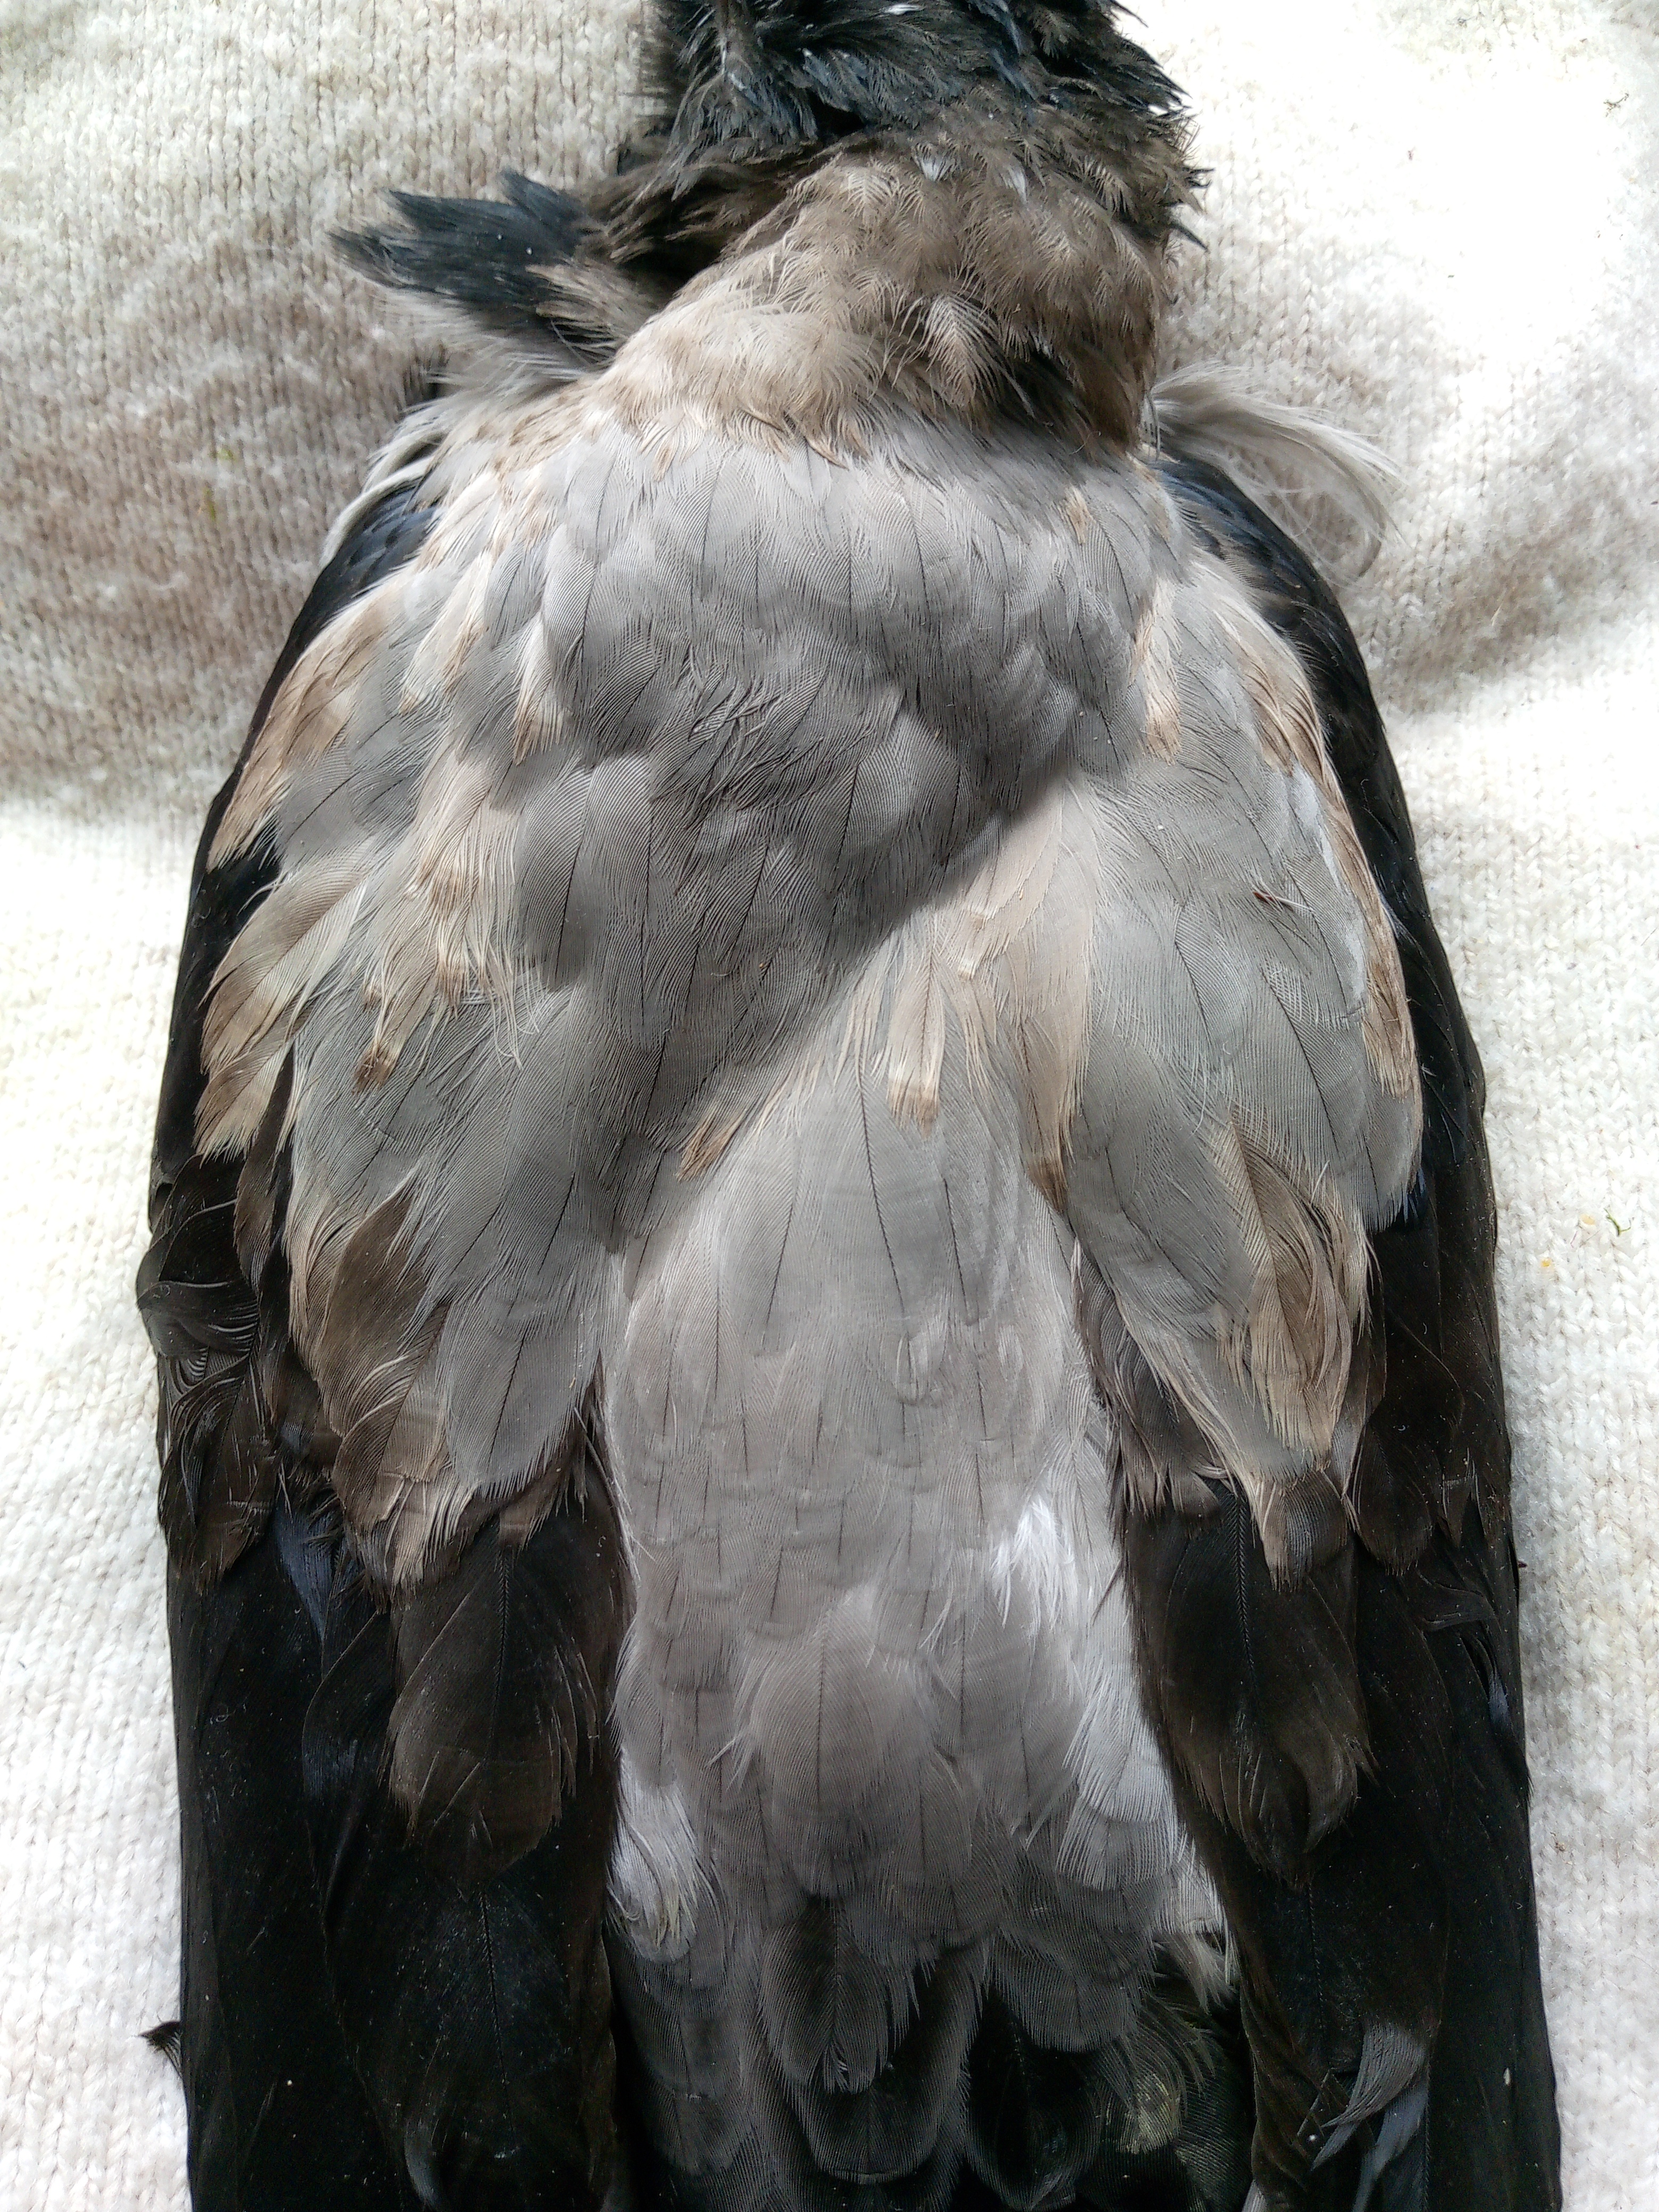
На изображении видны перья птицы (вероятно, серого голубя или вороны). На одном из перьев в центре заметен небольшой дефект, который напоминает механическое повреждение, след от укуса пухопероеда или деформацию стержня.
Возможные причины изменений структуры перьев у птиц:
Стресс-линии (островки голодания) — поперечные дефекты на опахале, возникающие из-за нехватки питательных веществ, болезней или сильного стресса в период роста пера.
Паразитарное поражение — активность эктопаразитов (например, пухопероедов), которые выедают бороздки, делая перо хрупким и «простроченным».
Механическая травма — залом или надрыв опахала из-за трения о прутья клетки, контакта с хищником или другими птицами.
Для точного определения проблемы и назначения лечения рекомендуется обратиться к ветеринару-орнитологу.
Рекомендации по уходу за оперением:
Полноценный рацион с добавлением серы и витаминов для птиц в период линьки.
Проверка кожи под перьями на наличие мелких ползающих насекомых.
Организация безопасного пространства без острых углов и тесных пространств.
Данная информация носит исключительно ознакомительный характер и не является заменой профессиональной ветеринарной помощи.
Если вы хотите узнать больше, уточните: птица живет дома или подобрана с улицы, а также присутствуют ли у нее зуд или выпадение перьев?
https://birds.vc/bolezni-ptitc/vorona-n … o.html/amp
https://www.jstor.org/stable/41477961
https://www.researchgate.net/publicatio … nsequences
Abstract and Figures
Fault bars are narrow malformations in feathers oriented almost perpendicular to the rachis where the feather vein and even the rachis may break. Breaks in the barbs and barbules result in small pieces of the feather vein being lost, while breaks in the rachis result in loss of the distal portion of the feather. Here, we provide a comprehensive review of 74 papers on fault bar formation in hopes of providing a clearer approach to their study. First, we review the evidence that the propensity to develop fault bars is modified by natural selection. Given that fault bars persist in the face of survival costs, we conclude that they must be an unfortunate consequence of some alternative adaptation that outweighs the fitness costs of fault bars. Second, we summarize evidence that the development of fault bars is triggered by psychological stress such as that of handling or predation attempts, and that they persist because the sudden contractions of the muscles in the feather follicle that control fright moults also causes the development of fault bars in growing feathers. Third, we review external and physiological (e.g. corticosterone) agents that may affect the likelihood that an acute stress will result in a growing feather exhibiting a fault bar. These modifying factors have often been treated as fundamental causes in the earlier literature on fault bars. Fourth, we then use this classification to propose a tentative model where fault bars of different severity (from light to severe) are the outcome of the interaction between the propensity to produce fault bars (which differs between species, individuals and feather follicles within individuals) and the intensity of the perturbation. This model helps to explain contradictory results in the literature, to identify gaps in our knowledge, and to suggest further studies. Lastly, we discuss ways in which better understanding of fault bars can inform us about other aspects of avian evolutionary ecology, such as the physiology of moult, the integration of moult into avian life cycles, and the strategies used to minimize stress during moult. Moreover, the study of fault bars may be relevant to understanding the aerodynamics of flight and the early evolution of flight.
Fault bars in bird feathers: mechanisms,
and ecological and evolutionary causes and
consequences
Roger Jovani1,∗and Sievert Rohwer2
1Department of Evolutionary Ecology, Estaci´on Biol´ogica de Do˜nana (CSIC), Avenida Americo Vespucio s/n, 41092 Seville, Spain
2Department of Biology and Burke Museum, University of Washington, Seattle, WA 98195, U.S.A.
ABSTRACT
Fault bars are narrow malformations in feathers oriented almost perpendicular to the rachis where the feather vein and even the rachis may break. Breaks in the barbs and barbules result in small pieces of the feather vein being lost, while breaks in the rachis result in loss of the distal portion of the feather. Here, we provide a comprehensive review of 74 papers on fault bar formation in hopes of providing a clearer approach to their study. First, we review the evidence that the propensity to develop fault bars is modified by natural selection. Given that fault bars persist in the face of survival costs, we conclude that they must be an unfortunate consequence of some alternative adaptation that outweighs the fitness costs of fault bars. Second, we summarize evidence that the development of fault bars is triggered by psychological stress such as that of handling or predation attempts, and that they persist because the sudden contractions of the muscles in the feather follicle that control fright moults also causes the development of fault bars in growing feathers. Third, we review external and physiological (e.g. corticosterone) agents that may affect the likelihood that an acute stress will result in a growing feather exhibiting a fault bar. These modifying factors have often been treated as fundamental causes in the earlier literature on fault bars. Fourth, we then use this classification to propose a tentative model where fault bars of different severity (from light to severe) are the outcome of the interaction between the propensity to produce fault bars (which differs between species, individuals and feather follicles within individuals) and the intensity of the perturbation. This model helps to explain contradictory results in the literature, to identify gaps in our knowledge, and to suggest further studies. Lastly, we discuss ways in which better understanding of fault bars can inform us about other aspects of avian evolutionary ecology, such as the physiology of moult, the integration of moult into avian life cycles, and the strategies used to minimize stress during moult. Moreover, the study of fault bars may be relevant to understanding the aerodynamics of flight and the early evolution of flight. Key words: bird flight, feather deformities, perturbations, physiology, stress.
CONTENTS
I. Introduction .............................................................................................. 2
II. Methods .................................................................................................. 3
III. Theoretical framework ................................................................................... 3
IV. Selection and the development of fault bars .............................................................. 3
V. Stressors that trigger the generation of fault bars ......................................................... 5
VI. Follicular mechanisms of fault bar formation ............................................................. 6
(1) Blood pressure ........................................................................................ 6
(2) Musculature contraction ............................................................................. 7
VII. Proximate factors shaping fault bar expression in individuals ............................................ 7
(1) Malnutrition .......................................................................................... 7
(2) Age and sex .......................................................................................... 8
(3) Disease ............................................................................................... 8
* Address for correspondence (Tel: +34 954 466 700; Fax: +34 954 621 125; E-mail: jovani@ebd.csic.es).
Biological Reviews (2016) 000– 000 ©2016 Cambridge Philosophical Society
2Roger Jovani and Sievert Rohwer
(4) Corticosterone ........................................................................................ 8
(5) Habitat ............................................................................................... 9
VIII. Overview ................................................................................................. 9
IX. Mechanistic model ....................................................................................... 10
(1) The model ............................................................................................ 10
(2) Empirical findings explained by the mechanistic model .............................................. 10
(3) Knowledge gaps revealed by the model .............................................................. 11
X. Ecological and evolutionary consequences of fault bars .................................................. 11
XI. Conclusions .............................................................................................. 12
XII. Acknowledgements ....................................................................................... 13
XIII. References ................................................................................................ 13
XIV. Supporting Information .................................................................................. 15
I. INTRODUCTION
Stressors produce growth abnormalities in keratin structures such as beaks, claws, feathers, hairs, hoofs or horns. In nails, for instance, these growth abnormalities have been traditionally associated with disease (Han et al., 2000; Ciastko, 2002), or intrusive medical treatments (Deliliers & Monni, 2001; Vassallo et al., 2001). However, they probably have little or no effect on individual fitness. A different picture arises when these growth abnormalities are produced in bird feathers.
Fault bars are feather malformations generated during feather growth (see pictures in Slagsvold, 1982; Murphy, Miller & King, 1989; Machmer et al., 1992; Sarasola & Jovani, 2006; Møller, Erritzøe & Nielsen, 2009). They vary from slight malformations that are difficult to see to extreme deficiencies in keratin deposition resulting in missing barbules and breaks in the feather vane and even the feather rachis (Riddle, 1908; Roest, 1957; Dawson, Bortolotti & Murza, 2001; Møller et al., 2009; Newton, 2010). Accordingly, many
studies classify fault bars by the severity of damage they may cause to feathers (often called ‘strength’, e.g. Sarasola & Jovani, 2006). Here we rank potential damage to feathers (fault bar severity hereafter) as light, moderate, and severe, according to how much the feather is weakened by the fault bar. Light fault bars resemble thin lines crossing the feather vein and appear, on close inspection, as a slight notch on the feather surface due to feather malformation (Sarasola & Jovani, 2006). Such fault bars rarely result in breaks in the feather vein and damage to the rachis amounts to only a slight discontinuity on the rachis surface, detectable
by sliding one’s fingernail along the rachis. Moderate fault bars consist of a conspicuous lack of keratin deposition in barbs and barbules (Murphy et al., 1989), making the feather translucent at the fault bar, and sometimes resulting in barbs that are bent at the fault bar. In this case the rachis often shows a clear malformation that is easy to see. Severe fault bars are seen as sections of feather vein a few mm wide that are free of barbules. Feather barbs often break at these fault bars, resulting in some loss of feather vein, and the rachis can also break causing loss of the distal part of the feather (Riddle, 1908; Roest, 1957; Newton, 2010).
Sebright (1826) seems to have been the first to discuss fault bars in his treatise on falconry, but Riddle (1907, 1908) and Duerden (1909) undertook the first serious investigations of the formation of fault bars. Since then, fault bars have attracted the attention of bird keepers (Ward & Slaughter, 1968; Taylor, 1991), veterinarians (Hudelson & Hudelson, 1995; Beynon, Forbes & Harcourt-Brown, 1996; Koutsos, Matson & Klasing, 2001; Koski, 2002; Rubinstein & Lightfoot, 2012) and ornithologists (e.g. Slagsvold, 1982; Murphy, King & Lu, 1988; Gombobaatar, Yosef & Birazana, 2009; Yosef, Gombobaatar & Bortolotti, 2013; Eggers & Low, 2014; Jovani, Montalvo & Sabat´e, 2014). Most research has focused on identifying the external and physiological factors that may stimulate the formation of fault bars and the proximate mechanisms by which the fault bars are generated during feather growth. More recently, a few studies have investigated how fault bar frequencies have been moulded by natural selection. Fault bars are oriented approximately perpendicular to the rachis (Riddle, 1908; Prum & Williamson, 2001; Maderson et al., 2009) and run parallel to the alternating light/dark feather growth bands that can be seen in some feathers and that usually record 24 h of feather growth (Brodin, 1993; Jovani & Diaz-Real, 2012). This leaves little doubt that they are generated by some trauma or perturbation affecting the collar cells of the feather follicle that generate the complex structure of growing feathers. This review shows that fault bars are costly and that the propensity of follicles to create fault bars can be reduced by natural selection. However, fault bars are still widespread in birds, thus challenging us to ask why they exist at all. We suggest that fault bars are a harmful by-product of some other adaptation carrying benefits that outweigh the costs of fault bars, as in the classic case of sickle cell anaemia conferring resistance to malaria in humans who are heterozygous for sickling (Ferreira et al., 2011). The aim of this review was to identify these other adaptations and to synthesize past research on fault bars by organizing them into a theoretical framework.
A recent review convincingly suggested that feather holes 0.5–1 mm in diameter (also called ‘fault spots’ by Murphy et al., 1989) may be related to fault bars (V ´ag´ asi, 2014). Previously, these holes were attributed to chewing lice (e.g. Møller, 1991). V´ag´ asi et al. (2011) found a positive correlation Biological Reviews (2016) 000– 000 ©2016 Cambridge Philosophical Society Fault bars in bird feathers 3 between the abundance of fault bars and feather holes among great tits (Parus major), but the same team (Pap et al., 2007) found these malformations to have different spatial distributions along the wing feathers within birds. This may suggest that fault bars and feather holes have different causes or that feather holes are less harmful and thus that their position along the wing of birds has been less shaped by natural selection. Pale bands, varying from a few millimetres to centimetres in width (see Murphy et al., 1988, 1989) are sometimes treated as fault bars. However, Murphy et al. (1988) found that synthetic diets deficient in sulfur-containing amino acids produced these pale bands without generating fault bars. Experimental studies in barn owls (Tyto alba) (Roulin et al., 2008) and feral pigeons (Columba livia) (Jenni-Eiermann et al., 2015) report increases in the frequency of pale bands in corticosterone-implanted birds (see Fig. 3 in Jenni-Eiermann et al., 2015), but they did not report the formation of fault bars. Although fault bars and pale bands are both feather malformations, they appear to have different proximal causes; thus, we advocate treating fault bars, feather holes, and pale bands as different phenomena (Pap et al., 2007; V ´ag´asi, 2014), while we encourage studying them simultaneously.
II. METHODS
We found relevant papers on fault bars by searching ISI Web of Knowledge and Google Scholar for word combinations such as fault bars, feather marks, fret marks, hunger traces, hunger faults, starvation marks, segmented dysplasia, stress bar, stress band or hunger streaks, and by snowballing, i.e. following references found in the papers we were reviewing. For each paper treating the formation of fault bars we noted the suggested cause or correlated factor (e.g. malnutrition, disease, age, sex), and the quality of the evidence provided. Evidence was considered ‘speculative’ in the absence of empirical data, ‘anecdotal’ when observations and analyses were few and when experiments lacked controls, ‘correlative’ when the occurrence of fault bars was related to potential causative factors, and ‘experimental’ when experimental and control treatments were reported.
We found 74 papers reporting 179 tests of hypotheses: 3.4% were speculative, 19.0% anecdotal, 60.3% correlative and 17.3% experimental (Table 1). A detailed account of each study is provided as online Supporting Information (Appendix S1), and synthesized in Table 1, and see online Tables S1 and S2.
III. THEORETICAL FRAMEWORK
The available literature identifies a number of potential stressors causing fault bars, many potential factors related to the abundance of fault bars, and two mechanistic hypotheses on how fault bars are generated by the collar cells of the feather follicle during feather growth. The likelihood of fault bars forming varies according to differences between feathers and feather tracts within individuals, differences among individuals related to age, habitat, and other factors, and differences among species. The temporal scale for factors that have been related to fault bar formation has also varied from seconds (handling), to hours (rain), days (malnutrition), months (disease), years (age), and beyond (natural selection). Past studies often seem to have mixed apples and oranges, emphasizing the need for a unifying framework to organize information on fault bar formation and persistence and, hopefully, to move this field forward.
We suggest that fault bar production should be studied on a time scale equivalent to the production of one fault bar in a particular feather follicle at a given moment. We further suggest that future studies clearly distinguish between (i) ultimate, evolutionary factors that shape the a priori propensity of an active feather follicle to generate a fault bar in response to a stressor; (ii) specific perturbations (stressors) that trigger the production of a fault bar at a particular moment; (iii) the mechanical or physiological mechanisms by which the feather collar cells actually generate a fault bar; and (iv) proximate factors that change the a priori propensity of fault bar generation at the individual level according to physiological and environmental factors.
We begin with a review of the literature on fault bars organized as suggested above. Next we present a mechanistic model linking these various levels of organization. Finally, we finish by discussing the link between fault bars and other physiological and life-history attributes of birds.
IV. SELECTION AND THE DEVELOPMENT OF FAULT BARS
The evidence that the propensity to develop fault bars can be modified by natural selection is strong, but mostly indirect. To be modified by natural selection, this propensity must be heritable, variable between individuals, and have fitness consequences.
As far as we are aware, only one experimental study demonstrates heritability of the propensity to develop fault bars. This study cross-fostered nestling barn swallows (Hirundo rustica) to evaluate the effects of vitamin E supplementation and brood size manipulation on nestling development (de Ayala, Martinelli & Saino, 2006). Neither of the two experimental treatments affected the incidence of fault bars in these nestlings, but the nest of origin had a strong and statistically significant effect on the incidence of fault bars in the rectrices of nestlings. This suggests that the propensity to develop fault bars has a heritable, genetic component, although maternal effects through the eggs cannot be excluded. Long-term fault bar pedigree studies (e.g. with an animal model approach) are encouraged to disentangle the environmental and genetic factors contributing to the formation of fault bars.
Table 1. Summary of the studies providing evidence for the different ultimate and proximate factors related to fault bar formation, as well as the mechanisms proposed and the stressors investigated. Proximate factors are variables differing between populations (e.g. habitat) or individuals (e.g. body size) within populations. Note that a single study can contribute to more than one hypothesis. Details for each specific test within each study can be found in the online Supplementary Information. Study categories are described in Section II
Effect: NO Effect: YES
Speculative Anecdotal Correlative Experimental Total Speculative Anecdotal Correlative Experimental Total Grand total
Ultimate issues
Genetic factors 1122
Inter-feather differences 1 1 6 13 19 20
Interspecific differences 22 44
Risk of feather damage 222
Species aerial foraging 111
Species aerial sexual displays 1 1 1
Species diet 1 1 1
Species domestication 1 1 1 1 2
Species flight 111
Species hybridization 1 1 1
Species migration 111
Species predation pressure 111
Species sexual dichromatism 1 1 1
Survival 1 1 5 5 6
Total 0 2 5 0 7 1 10 25 1 37 44
Proximate factors
Age 1 1 1 13 14 15
Arrival date 1 1 1
Body condition 2 2 1 1 2 4
Bodysize 11 112
Breeding effort 1 1 1
Broodsize 11 112
Clutch size 1 1 1
Colony size 111
Corticosterone 1 1 4 4 5
Cost of ornaments 2133
Crowding 1 1 1
Disease 1 1 2 1 4 1 6 8
Egg size 1 1 1
Fluctuating asymmetry 1 1 1
Habitat 2 2 6 6 8
Hatching date 1 1 1
Hour 121 44
Interspecific competition 111
Inter-individual differences 111
Laying date 111
Malnutrition 1 3 10 14 1 7 1 4 13 27
Need for fast moult 1122
Nestling rank 1 1 1 1 2
Other feather defects 1 3 4 1 1 2 6
Plumage features 1 1 2 2 3
Sex 6 6 5 5 11
Total 0 3 28 12 43 3 12 48 7 70 113
Mechanisms
Follicle nutrition 111
Follicle collapse 1 1 1
Musculature contraction 1 1 1 1 2 3
Total 0 0 0 1 1 2 2 0 0 4 5
Stressors
Altrazine (herbicide) 1 1 1
Environmental change 111
Food unpredictability 111
Handling 2 2 1 1 5 7 9
Psychological stress 222
Weather 1 1 2 1 1 3
Total 031 15021 91217
Grand total 0 8 34 14 56 6 26 74 17 123 179
Fault bars in bird feathers
Although evidence is limited (and more longitudinal studies are encouraged), individuals have been shown to vary in their likelihood of developing fault bars across successive moults. Thus, American kestrels (Falco sparverius) varied consistently across years in the numbers of fault bars they developed, suggesting variation among individuals in the propensity to develop fault bars (Bortolotti, Dawson & Murza, 2002). If these differences have a genetic component, as the barn swallow study suggests, then the propensity to develop fault bars could be modified by selection.
The fitness costs of fault bars seems clear. Feathers break at fault bars and broken feathers are generally not replaced until the next scheduled normal moult of the feather. Thus, the fitness consequences of broken feathers could last up to several years in large birds with incomplete moults (Rohwer et al., 2009). Reductions in wing area increase wing loading, which reduces flight performance (Velando, 2002; Navarro & Gonz´alez-Solís, 2007). Fitness costs of fault bars have been shown in several studies. Each fault bar in the rectrices of both willow tits (Poecile montana) and crested tits (Lophophanes cristatus) was associated with a 5% reduction in survival (Eggers & Low, 2014). Three other studies reported higher mortality among birds with more fault bars. Juvenile great tits with more fault bars were significantly less likely to be recaptured than those with fewer fault bars (Pap et al., 2007). Juvenile Siberian jays (Perisoreus infaustus) with more fault bars in their primaries were more likely to be killed by predators in their first winter (Griesser, Nystrand & Ekman, 2006). Finally, feathers of prey species taken by goshawks (Accipiter gentilis) and sparrowhawks (Accipiter nisus)weremorelikely to contain fault bars than were netted individuals of those same prey species, suggesting that individuals with more fault bars were more susceptible to predation (Møller et al., 2009); measures of condition were not related to numbers of fault bars in the 47 prey species they examined. It is important to note that none of these studies distinguishes between the direct cost of fault bars and the alternative that fault bars merely identify individuals in poor condition that were less likely to survive for reasons unrelated to the fault bars in their plumage. That would require experiments.
Current evidence suggests that natural selection shapes the propensity of feather follicles to develop fault bars at two levels: between bird species, and according to feather position within individual birds. Bird species differ greatly in their abundance of fault bars (Taylor, 1991; Freed, Medeiros & Bodner, 2008; Møller et al., 2009). For instance, nestlings of many species have more fault bars than adults (e.g. Jovani & Tella, 2004; Eggers & Low, 2014), but there are species, such astheEuropeanpiedflycatcher(Ficedula hypoleuca), where nestlings are largely free from these malformations (Kern & Cowie, 2002). These differences in fault bar propensity among species seem to be related to species characteristics that make fault bar expression more or less penalized by selection. For instance, ostrich (Struthio camelus) farmers find it difficult to produce wing feathers without fault bars, presumably because flightlessness makes the expression of fault bars less costly in ostriches (Duerden, 1909). More recently, Møller et al. (2009) found that birds that fly differ greatly in fault bar prevalence and abundance, with species that suffer higher predation pressure or that have longer migrations showing fewer fault bars. From these results they concluded (p. 343) that ‘ ... developmental control or susceptibility to stress can change when intensity of natural selection changes’.
Differences in fault bar abundance between feathers within individuals (even contiguous feathers of the same feather track) also suggest that natural selection has shaped the propensity to develop fault bars. Thus, fault bars are symmetrically distributed in the left and right rectrices of juvenile ospreys (Pandion haliaetus; Machmer et al., 1992) and juvenile barn swallows (Serrano & Jovani, 2005). Because juvenile rectrices grow simultaneously and, thus, experience the same stressors, the left–right symmetry in the distribution of fault bars in the tail clearly shows that the propensity to develop fault bars differs between contiguous feather follicles. These differences presumably result from selection opposing fault bars in feathers where breaks in the vein or rachis would affect fitness more seriously (e.g. by being more important for flight).
This ‘fault bar allocation’ hypothesis is supported in studies reporting that rectrices regularly have more fault bars than remiges (Slagsvold, 1982; Bortolotti et al., 2002; Sarasola & Jovani, 2006), and inner remiges more than outer remiges (Murphy et al., 1989; Jovani & Blas, 2004; Pap et al ., 2007; Jovani et al., 2010). Relative to rectrices and secondaries selection apparently has suppressed the occurrence of fault bars in the primaries, perhaps because they experience greater strain during flight (Jovani & Blas, 2004). In both raptors and cranes fault bars are less common in primaries than in rectrices or secondaries but they are more likely to result in feather breaks in the primaries when they occur there (Sarasola & Jovani, 2006; Jovani et al., 2010). This pattern suggests that natural selection has suppressed the production of fault bars in feathers where damage would seriously lower survival. Indeed, Pap et al. (2007) found that juvenile great tits were less likely to be recaptured if they had more fault bars in their primaries but not if they had more in their secondaries and tertials.
V. STRESSORS THAT TRIGGER THE GENERATION OF FAULT BARS
Fault bars are a punctuate phenomenon, thus it seems logical to suspect that fault bars are triggered by some factor occurring during a short period of time or, at least, that the processes that produce fault bars occur during a short time in the follicle collar of a growing feather.
While studying the energetic and nutritional demands of moulting in the white-crowned sparrow (Zonotrichia leucophrys gambelii), King & Murphy (1984) and Murphy et al . (1988) made a serendipitous discovery: fault bars were created on the days when they handled the birds, in both control and experimental birds. They concluded that: ‘We think that the weight of evidence strongly favors the shock of handling as the cause of fault bars in captive birds, and presumably some similar shock (such as flight from a predator) causes them in free-living birds’ (King & Murphy, 1984, p. 169). Later experiments confirmed these results, and led the authors to suggest that fault bars are a mild form of the response to shock that produces fright moult, the instantaneous shedding of feathers when birds are stressed such as during a predatory event (Murphy et al., 1988, 1989).
The link between being restrained by a researcher, or a similar stress such as a failed predation event, and fault bar formation is supported by other studies. Negro, Bildstein & Bird (1994) found that hand-reared nestling American kestrels developed more fault bars than parentally reared nestlings, irrespective of whether hand-reared nestlings were fed ad libitum or not. While this does not discount other factors (and note that food delivered by parents to naturally reared nestlings was not manipulated), this study suggests that the psychological stress of not being with their parents and being handled by researchers contributed to the formation of fault bars. Whitmore & Marzluff (1998) found a similar result (but including an effect of malnutrition) in hand-reared corvids of three species.
Other psychological factors have been studied as causes of fault bars. In an interesting experiment using captive European starlings (Sturnus vulgaris) Strochlic & Romero (2008) compared controls (no stress) with three experimental stress groups: 30 min of chronic stress four times a day, acute stress of being handled for 30 min, and chronic stress with food restriction. Although controls and stress groups did not differ significantly in numbers of fault bars on a single rectrix (P=0.08), the chronic and acute stress treatments had three to fivefold more fault bars than the controls; non significance may have resulted from small sample sizes. A recent study of house sparrows (Passer domesticus) showed higher stress responses (corticosterone levels) in young birds than in adults when they were handled by researchers and that the stress response of young birds declined as they grew (Lendvai et al., 2015). This is interesting because young birds consistently have more fault bars than adults (see Section VII.2), which, again, is consistent with fault bars having a psychological cause. Overall, current evidence suggests that handling, and other similar acutely frightening stressors, like predation attempts, are powerful triggers of fault bar production. In fact, even predation exposure without actual predation attempts has been related to fault bar formation (see Section VII.5).
VI. FOLLICULAR MECHANISMS OF FAULT BAR FORMATION
A major gap in our understanding is that we do not know how fault bars are generated in growing feathers by the feather follicle (Prum & Williamson, 2001; Maderson et al., 2009). Whether fault bars are created by some mechanical force, or by a change in the physiology of the follicle collar cells, or by a combination of the two is unclear.
(1) Blood pressure
Riddle (1907, 1908) suggested that fault bars are formed by reduced blood pressure in the follicle collar during the first hours of night. He suggested that this reduced nutrition to the growing feather, resulting in reduced keratin deposition and a fault bar. Riddle tested this hypothesis by starving captive birds, and treating them with amyl nitrite and other substances thought to decrease blood pressure, but support was ambiguous. Duerden (1909) proposed an alternative, also based on blood pressure. Rather than positing a shortage of nutrients (a physiological cause), he suggested that a reduction of blood pressure inside the developing feather during the early hours of the night would cause mechanical collapse of the feather follicle, like sucking a blocked straw, resulting in the generation of a fault bar. Duerden (1909, p. 479) thought that reduced blood pressure was sufficient to mechanically collapse the sheath of the growing feather: ‘From long observation every farmer [of ostriches for the production of feathers] knows, even before the plumes unfold, that bars will be present wherever the outer sheath is indented, while if the sheath is smooth all the way the feathers will be faultless’. Note, however, that these indentations in the feather sheath could equally be the result of muscles in the feather follicle suddenly contracting during the stress of being handled or frightened by a predator, both of which cause fault bar formation (see Section 5).
These blood pressure-related hypotheses suggest that fault bars are mainly generated in the early part of the night when blood pressure is reduced; thus, no more than one fault bar should be generated every 24 h, implying that consecutive fault bars in the same father should be separated by the length of feather grown during 24 h (i.e. the width of a pair of light–dark growth bands). Riddle (1907, 1908) and Duerden (1909) reported this to be the case, as did Jovani & Diaz-Real (2012); however, the latter authors found that many fault bars developed at other hours, particularly in adult birds. Murphy et al. (1989) assessed the blood pressure hypothesis more directly by showing the night-time blood pressure reduction to be slight and unlikely to be sufficient to collapse the feather follicle and induce a fault bar. Thus, the hypothesis of reduced blood pressure has little empirical support. However, the possibility that fault bars are mostly generated during certain parts of the diel cycle (e.g. during the first hours of the night in white stork, Ciconia ciconia, chicks: Jovani & Diaz-Real, 2012) merits further study as it may facilitate understanding the proximal mechanisms of fault bar formation.
From an evolutionary perspective, reductions in blood pressure could generate fault bars if the reduction in blood pressure was an adaptive response to stressors. For example, cold stress might reduce peripheral blood flow and pressure to conserve heat and lower the cost of feather production. However, the ‘musculature contraction’ hypothesis (see Section VI.2) is more likely because predation attempts can cause fault bars to form (King & Murphy, 1984; Murphy et al., 1988) and the mere sight of a hawk raises blood pressure in turkeys (Krista et al., 1981), rather than lowering it.
(2) Musculature contraction
King & Murphy (1984) and Murphy et al. (1988) suggested that fault bars are created by a sudden contraction of the musculature around the soft feather follicle during feather growth (Homberger & de Silva, 2003; Maderson et al., 2009). King & Murphy (1984) cite Dathe (1955) to support this notion, but the latter author could not decide if the feathers lost in fright moults were lost by sudden contraction or relaxation of these muscles. We assume that strong contractions are the underlying mechanism because feathers are also attached to the skin by connective tissue that would prevent them from being extruded solely by relaxation of the muscles surrounding the follicle.
King & Murphy (1984) noted that the nonstriated muscles surrounding the feather follicle were probably powerful enough to crimp the feather sheath and cause the generation of a fault bar. In experimental oil-filled feather follicles inserted into the sockets of plucked feathers pressures generated by the stimulation of these muscles averaged 2.4-fold above baseline pressure and, in some experiments, reached fourfold above baseline (Peterson & Ringer, 1968). Murphy et al. (1989, p. 1317) conclude that ‘fault bars may result from unusual contractions of feather muscles that are normally inhibited while a feather is growing and its sheath is soft’. These muscle contractions could also account for the indented sheaths in the feathers of ostriches always resulting in fault bars (Duerden, 1909).
The beauty of the suggestion by Murphy et al. (1989), that fault bars are generated by involuntary contractions of these feather muscles, is that they attribute these sudden contractions to an alternative fitness benefit, fright moults, which clearly seem to benefit birds escaping from predators (Dathe, 1955; H¨oglund, 1964). Consideration of genetic correlations as the cause of maladaptive traits did not characterize thinking when Riddle (1908) and Duerden (1909) were writing, but it is clear that Murphy et al. (1989) were thinking in these terms in their interpretation of the development of fright bars. Thus, they posit that the loss of feathers in fright moult and the involuntary development of fault bars during the growth of feathers were both caused by contractions of the muscles surrounding the feather follicle. The implication is that inhibition of this muscular contraction cannot be complete in those species where fright moult generates a fitness benefit that exceeds the fitness cost of fault bars generated by sudden stressors that cause the contraction of these muscles while feathers are growing. This is consistent with their strong experimental evidence that handling stress causes fault bars and, further, does so much more frequently in naïve than habituated birds (King & Murphy, 1984; Murphy et al., 1988). However, Murphy et al. (1989) also acknowledge Riddle’s (1908) circumstantial evidence that unsuccessful begging or foraging, odd smells, and food adulterants may also stimulate formation of fault bars. We consider these other factors as general stressors affecting the propensity to develop fault bars, rather than stimuli that might cause contractions of the feather muscles.
To test the idea that fault bars are an unfortunate consequence of the ability to undergo fright moults, we need experiments exploring whether artificial stimulation of the follicular muscles can produce fault bars in growing feathers, and whether the stimulus needed to generate these contractions varies according to differences among species in their propensities to undergo fright moults. The latter could be investigated by relating the frequency of fault bars seen in rectrices to the index of the propensity to show fright moults developed by Møller, Nielsen & Erritzøe (2006), which is simply the difference in the force required to pluck rump feathers compared to feathers from the upper back or breast. That rectrix feathers are frequently lost in fright moults (Juhn, 1955; Møller et al., 2006) and that they regularly have far more fault bars than remiges (Møller et al., 2009) is consistent with fright moults and fault bars having a common cause that inversely links their fitness costs and benefits.
VII. PROXIMATE FACTORS SHAPING FAULT BAR EXPRESSION IN INDIVIDUALS
So far, we have established two general principles. First, species and feather groups differ in their propensity to develop fault bars in ways that suggest adaptive responses to the survival costs imposed by fault bars; and second, the immediate stressor triggering the formation of a fault bar seems to be some form of acute fear. Below we review a series of proximate factors that can modify the propensity for an acute stressor to trigger the formation of a fault bar in a growing feather. Much of the earlier literature treating these factors has not distinguished between treating them as fundamental causes of fault bars and treating them as modifiers of the propensity to produce fault bars. Thus we emphasize that we are treating these factors as modifiers of the likelihood that a follicle will produce a fault bar in response to a triggering stress. These modifying factors may be intrinsic, such as sex, age or developmental history, or extrinsic, such as food availability, disease or habitat features, but there is little evidence that they are able to generate fault bars in the absence of a triggering stimulus.
(1) Malnutrition
Malnutrition was likely the first factor to be related to fault bars (Sebright, 1826), leading to fault bars being called ‘hunger traces’ or ‘hunger streaks’. Riddle’s (1907, 1908) pioneering studies suggested that malnutrition was a key factor in explaining fault bar formation, with the result that it has been examined in no less than 27 studies, 14 of which are experimental (Table 1). While some evidence supports this hypothesis (e.g. Waite, 1990), 10 out of 14 experimental tests of hunger as a proximate modifier of the propensity to develop fault bars failed to induce fault bar formation through food restriction or malnutrition (Table 1; e.g. King & Murphy, 1984; Murphy et al., 1988; Negro et al ., 1994; Searcy, Peters & Nowicki, 2004). Thus, current empirical evidence fails to show that malnutrition strongly modifies the propensity for fault bars to form.
Related to malnutrition is general body condition. Although current evidence (Table 1) does not suggest condition to be strongly correlated with the propensity to develop fault bars, body condition cannot be ruled out completely. Condition, measured as mass corrected for size, was related to fault bar frequency in American kestrels (Bortolotti et al., 2002). Fault bar abundance has also been related to features linked to differences in body condition among individuals, such as nestling rank or number of nestlings in a brood (Machmer et al., 1992; Gombobaatar et al., 2009), or co-occurrence with other kinds of feather defects (Harrison, 1963) or feather secondary sexual characters (V´ag´asi, Pap & Barta, 2010; V´ag´asi et al.,2012). Further, individuals with better developed sexual ornaments often have fewer fault bars (Møller, 1989, 1994; Blanco & de la Puente, 2002; but see Andersson, 1994), which is consistent with those individuals being in better condition. Interestingly, five out of six studies have shown that individuals with more fault bars have lower survival (Table 1). While fault bars may directly explain lower survival in some cases by impairing flight and the ability to escape predators, it is perhaps more likely that fault bars merely identify lower quality individuals that would be less able to escape predators, even without fault bars. Only experiments can sort this out.
(2) Age and sex
While sex does not appear to affect fault bar formation, age is strongly associated with fault bar frequency (Table 1). Younger birds consistently have more fault bars than older conspecifics, both across individuals (Slagsvold, 1982; Blanco & de la Puente, 2002; Jovani & Blas, 2004; Jovani et al., 2014) and within individuals developing from nestling to adult plumage (Pap et al., 2007; Leloutre, Gouzerh & Angelier, 2014). Indeed, age even affects the development of fault bars within developing nestlings, as studied by the position of fault bars along growing feathers (Machmer et al., 1992; Jovani & Tella, 2004; Jovani & Diaz-Real, 2012). Jovani & Tella (2004) found an exponential decrease in fault bar formation during nestling growth, which paralleled the increase in survival of nestlings with age; young that are less able to confront environmental perturbations produce more fault bars.
(3) Disease
Disease also predicts differences in the propensity to develop fault bars in some studies. Male house sparrows with many fault bars had relatively larger bursas of Fabricius, which indexes the severity of parasite infections (Møller, Kimball & Erritzøe, 1996). Similarly, Freed et al. (2008) found more fault bars in individuals infected with chewing lice in nine avian species. Jovani et al. (2014) found a clear correlation between Campylobacter enteric bacterial infection and fault bar abundance in feral pigeons, suggesting either a causal relationship or (more likely) a higher propensity to develop fault bars among physiologically compromised birds. Manniste & Horak (2014) reported similar results for captive greenfinches (Carduelis chloris) that died from Trichomonas infections.
A study by Romano et al. (2011) is possibly the most interesting. They treated nestling barn swallows with bacterial lipopolysaccharide (LPS), thus simulating a bacterial infection without the detrimental costs of actual infections and found both the prevalence and abundance of fault bars to be about twice as high in experimental than in control nestlings. Moreno-Rueda (2010) found that LPS-injected birds had a slower moult speed than controls, thus suggesting a link between LPS injection and feather regeneration physiology. Because LPS, per se, could not explain the production of fault bars, he suggested that the higher corticosterone titres associated with LPS treatment (Owen-Ashley et al., 2006) might be responsible for the additional fault bars because high corticosterone levels have been related to reduced feather quality (see Section VII.4).
(4) Corticosterone
Corticosterone, the predominant avian glucocorticoid and a hallmark of the adrenocortical response to stress in birds (Blas, 2014), has attracted substantial attention in relation to feather moult physiology (e.g. Romero, Strochlic & Wingfield, 2005; DesRochers et al., 2009; Almasi et al ., 2012; Jenni-Eiermann et al., 2015). Corticosterone has complex, contrasting and even opposing effects when related to food intake and feather growth. For instance, Patterson et al. (2014) found more corticosterone in feathers of nestling Caspian terns (Hydropogne caspia)fedad libitum compared to conspecifics ingesting only two-thirds the amount of food, while Will et al. (2014) found higher feather corticosterone in food-restricted rhinoceros auklets (Cerorhinca moncerata) that were hand-reared or manipulated in the field. Almasi et al. (2012) found corticosterone implants to reduce feather growth rate in nestling barn owls, resulting in shorter wing lengths at fledging. Similarly, Romero et al. (2005) found that corticosterone-implanted European starlings grew feathers more slowly than controls. DesRochers et al. (2009) found that both endogenous (experimentally increased by psychological stress) and exogenous (increased with implants) sources of corticosterone reduced feather quality in European starlings, particularly in rectrices. However, Fairhurst et al. (2014) found a negative correlation between corticosterone levels and the formation of fault bars in wild common redpolls (Acanthis flammea); moreover, feathers with higher corticosterone levels had wider growth bands and those birds had redder plumage, both of which may suggest that corticosterone enhances food finding and the mobilization of body stores for feather growth.
Much less is known about the role of corticosterone in the production of fault bars (Table 1). Using radioimmunoassay, Bortolotti et al. (2009) found more corticosterone in feather segments with one or more fault bars than in adjacent feather segments without fault bars. Also, Patterson et al. (2014) showed corticosterone levels to be higher in the distal parts of feathers, which grow first, in Caspian tern chicks, a pattern that is consistent with fault bars being more frequent in the distal parts of the feathers in nestling raptors and storks (Machmer et al., 1992; Jovani & Tella, 2004; Jovani et al., 2014). Among other physiological actions, elevated plasma corticosterone levels are known to increase protein catabolism (Blas, 2014), potentially reducing keratin synthesis during feather growth, which could lead to fault bar formation. Fokidis et al. (2012) found that captive curve-billed thrashers (Toxostoma curvirostre) provided with an unpredictable food supply elevated their initial (baseline) plasma corticosterone, but decreased their stress-induced levels (in response to 30 min of handling and restraint) compared to control birds with constant access to food. Interestingly, birds in the variable-feeding group developed five times more fault bars, which may suggest that baseline, but not stress-induced, corticosterone elevations induced fault bar formation.
Overall, corticosterone is a promising candidate mediator between environmental perturbations (e.g. weather, predation risk, actual predation attempts) and other proximate factors of fault bar production (e.g. age, disease). However, much more research is needed to understand the role of the hypothalamic–pituitary–adrenal axis on feather development in general, and on fault bar formation in particular. For example, no study has tested the effects of other avian hormones involved in the adrenocortical response to stress [e.g. corticotropin-releasing hormone (CRH), arginine vasotocin (AVT), adrenocorticotropic hormone (ACTH)] on fault bar formation (J. Blas, personal communication). Some of these hormones could have a more direct role in fault bar production than corticosterone, such as disrupting cell membrane physiology, which might not allow the accumulation of keratin, or altering cell to cell adhesion in the follicle collar, which could induce keratinocytes to separate during feather generation and create a fault bar.
Again, the evolutionary interpretation of a potential role of corticosterone in the production of fault bars would be that increases in blood titres of corticosterone are a beneficial stress response, and that fault bars are either the unavoidable consequence of this stress response or that reduced keratin deposition mediated by corticosterone is a stress response that lowers energy consumption by processes such as feather growth that are not vital in an emergency situation. More studies on the role of corticosterone on the formation of fault bars are strongly encouraged.
(5) Habitat
Habitat features may also change fault bar propensity. In a fully crossed experimental design Witter & Lee (1995) found a higher occurrence of fault bars in captive European starlings housed in cages without cover; treatments were cages with or without vegetation cover and food positioned near or far from the cover. The authors suggested that the perceived risk of predation in the habitat was behind fault bar abundance. In addition, differences have been reported between habitats in six out of eight correlative studies on fault bar occurrence (Table 1), and most of these studies argued that habitat resources (mainly food) were behind these results. While food differences may actually be a causal factor in some of these studies (e.g. Blanco, Laiolo & Fargallo, 2014), we are more inclined towards the interpretation of Witter & Lee (1995) that psychological stress linked to reduced vegetation cover and increased risk of predation may underlie these results. In fact, correlative studies seem to support this hypothesis because birds carried more fault bars in regenerating forests (Sodhi et al., 2005), in habitats with less vegetation cover (Griesser et al., 2006; Eggers & Low, 2014), and in more fragmented habitats (Sodhi, 2002). Similarly, Fokidis et al. (2012) found that the same amount of food delivered to captive birds increased the number of fault bars if it was delivered in an unpredictable way. It would appear that psychological factors, and not resource abundance, per se, could explain the differences between habitats.
VIII. OVERVIEW
So many specific factors affect the expression of fault bars that a brief overview of some of the more important trends in Table 1 seems merited. Concerning ultimate, selective factors, differences between feather tracts in the prevalence of fault bars have been recorded in 19 of 20 studies, strongly attesting to selection having modified the propensity of different feather groups to form fault bars. The high prevalence of fault bars in the rectrices is consistent with predation attempts being the primary stressor causing their formation and the rectrices often being ejected in fright moults. There is a surprising shortage of studies reporting species differences (N=4) and relating fault bar prevalence with species predation pressure (N=1); however, five of six studies have found individuals with more fault bars to be less likely to survive. Concerning proximate factors that modify the likelihood that a stressor will result in the formation of a fault bar, age is the only clearly confirmed factor, with 14 of 15 studies showing young birds to have more fault bars than adults. However, three additional contingencies have reasonable cross-study support for affecting the likelihood of fault bar expression: corticosterone, disease, and habitat. Sex and malnutrition have been addressed in good numbers of studies but neither factor seems clearly associated with fault bar formation. Table 1 also clearly demonstrates the serious shortage of studies treating the specific follicular mechanism that generates fault bars in growing feathers. Current understanding suggests that the most likely mechanism is strong contraction of the follicular muscles associated with fright stress, but this awaits further study. Finally, of the specific stressors that may generate fault bars, only handling stress has been reasonably well studied, with seven of nine studies finding an effect of observer handling, which presumably resembles the stress of a predation attempt.
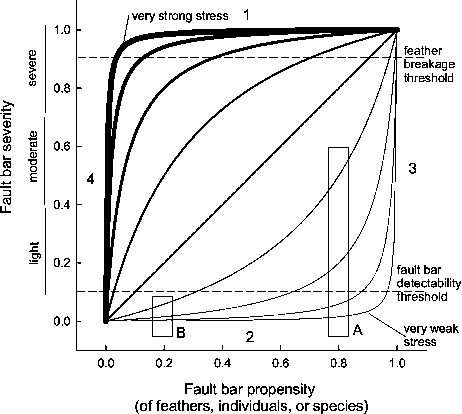
Fig. 1. Model of the interaction between propensity of a feather follicle to produce fault bars (x-axis), the strength of the stressor (plotted lines) and the resulting fault bar severity (y-axis). Note that the x-axis may account for different scales (differences in fault bar propensity between feathers, individuals or species). Fault bar propensity is shaped by ultimate (see Section IV) and proximate (see Section VII) factors. See Section IX for explanation of numbers (1–4) and letters (A, B).
IX. MECHANISTIC MODEL
Отредактировано Au (30-08-2026 19:12:22)
Поделиться76128-08-2026 15:19:11
- Администратор
- Откуда: Sol III
- Зарегистрирован: 30-07-2011
- Сообщений: 52239
- Пол: Мужской
- Провел на форуме:
1 год 4 месяца - Последний визит:
Сегодня 22:04:10
Это все водилы
ой, даладна.. вот прям каждый водила имеет НЕСКОЛЬКО ДЕСЯТКОВ ДТП..
эти ЫЫшные боты совсем уже потеряли берега со своим ЫЫ-маркетингом 
Поделиться76230-08-2026 20:08:38
- Активный участник
- Зарегистрирован: 25-07-2011
- Сообщений: 13988
- Провел на форуме:
4 месяца 19 дней - Последний визит:
02-09-2026 08:45:14